

Last week, I attended the tail end of a Keystone conference on Epigenetic Regulation of Aging, followed by a one-day brainstorming session to kick off a project called GILGA-mesh, intended to take this bull by the horns. Though the subjects of the two days were virtually identical, the approach and attitudes of the scientists in attendance set very different tones. Both days featured smart, creative and careful scientists, but they saw the same material through different frameworks. Sometimes philosophy makes a difference.
For readers who know me less well, I should introduce my perspective: I believe that aging is an evolved epigenetic program. When we are young and growing, particular genes are turned on and off with exquisite timing to determine the growth and development of bones, muscles, and organs. When we are old, the program continues, more slowly and more diffusely, but inexorably nonetheless. Genes are turned on that destroy us with inflammation and cell senescence and auto-immunity and programmed cell death, while the systems that protect us from pathogens and from free radical damage are gradually shut down. Evolution has left nothing to chance.
[I first wrote an academic paper about this idea in 2013, excited by a paper by Adiv Johnson on methylation, but unaware that Tom Rando had written on the same lines the previous year. Jeff Bowles had hinted at similar ideas in a paper more than a decade earlier. Soon the field was broken wide open by the work of a bio-statistician.
Steve Horvath ran a computer analysis on thousands of genes as they are expressed in young and old humans, and produced an “epigenetic clock” that could accurately report how old a person using measurementis of methylation in 353 DNA sites in particular.]
Background
Epigenetics is a new science in the 21st century. All the cells in one body have the same DNA (pretty much), but differernt genes are “expressed” (translated into proteins) in different tissues and at different times, and this is what controls the body’s metabolism. In fact, only 2% of our DNA is genes, and 98% determines how the DNA is folded and spooled, opened and closed at particular times and places, and this in turn controls gene expression. We are 2% genetic and 98% epigenetic.
There is a language called the “genetic code” which determines how genes are translated into proteins. It was decoded by Francis Crick and others in the 1950s. It is as simple as it can be, and is completely understood. There is another language, the “epigenetic code” that determines gene expression. It is anything-but-simple, with a convoluted and self-referential syntax that we are just beginning to understand. The epigenetic code starts with signals embedded in the DNA that serve as “start” and “stop” codons. The stretch in between comprises a piece of a gene, a kind of Gutenberg movable type that is transcribed from the chromosome and then spliced and combined to form functional RNAs and proteins. The complicated part of the epigenetic code is implemented as a pattern of methyl and acetyl groups. These are little chemical decorations that attach to the DNA and to the “histones” (spools around which DNA is wound up in the cell nucleus for safe storage). The methyl and acetyl groups are continually being attached and removed according to instructions that come from within the cell and other instructions that are passed through the blood. It is the methyl and acetyl groups that determine how the DNA is folded and spooled, which effectively turns particular genes on and off as needed.
The part of the epigenetic code on which we have the best handle at present is called “methylation of CpG islands”. Long stretches of DNA have CGCGCGCG… on one strand, complemented by GCGCGCGC… on the other. Often the C’s in this region get an extra methyl group, turning from cytosine to 5-methylcytosine. Then this stretch becomes a “repressor region,” a signal to NOT express the adjacent gene.
DNA methylation can be persistent, turning a gene off for decades at a time. When a cell divides and its DNA is copied, the methylation pattern can be copied with it. This accounts for some of the persistence of epigenetics, and the way gene expression can be inherited across generations.
DNA methylation has been appreciated for 30 years, but two recent developments make the subject attractive and accessible to research. (1) There is now a simple lab/computer technique for reading the methylation pattern from DNA. It relies on commercially available, automated machinery for PCR to sequence a full genome before and after chemical modification of the methylated C’s. (2) There is now a simple lab/computer technique for changing the methylation state of any chosen target site in the DNA. It is based on CRISPR technology that is taking genetics labs by storm the last two years.
Epigenetics and aging
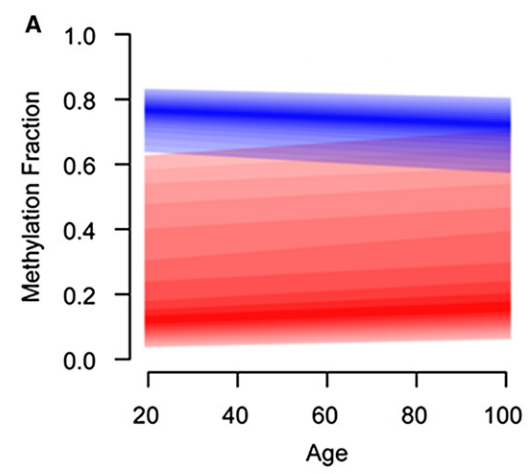
Three years ago, Horvath demonstrated that there are specific patterns of methylation associated with particular ages of the body. It’s not just that the fresh, clear pattern of youthful gene expression becomes muddied and random with age—although there is some of that. But it’s also true that some genes that are active in youth become inactive as we get older and (especially) that other genes that were suppressed in youth become activated in old age. What Horvath’s paper says is, “show me methylation pattern of a person’s cells, and I can tell you how old s/he is.”
Is epigenetics a cause or effect of aging?
The correlation between aging and epigenetic status is established beyond dispute. But what does it mean? This is the big question. Most researchers think of the body as programmed by evolution to be as strong and healthy as possible. So, when different genes are expressed in old age, they find it natural to assume that the body is protecting itself in response to damage that it has suffered over the years. We express different genes when we are older because we need different genes when we are older. This was the predominant attitude at the first conference (where I was present just for the last day).
The other possible interpretation is my own, and it has become common among those who are closest to the field of epigenetics. It is that epigenetic changes with age are means of self-destruction. The body is programmed to die, and its suicide plan is laid out in the form of transcribing an unhealthy combination of genes. This idea flies in the face of traditional evolutionary theory. (How could natural selection prefer a genome that destroys itself and cuts off its own reproduction?) Nevertheless, the evidence for this hypothesis is robust. The genes that are turned on don’t protect the body—quite the opposite. Genes for inflammation are dialed up. Genes for the body’s defense against free radicals are dialed down. Cell turnover is dialed down. DNA repair is dialed down. The mechanisms of programmed cell death (apoptosis) are strengthened in healthy cells, at the same time that they are perversely weakened in cells that are a threat to the body, like infected cells and cancer cells.
How will we determine who is right?
In my opinion, the existing evidence heavily favors the hypothesis that aging is caused by epigenetic changes, rather than the other way around. When we look at the kinds of changes that occur, they seem to be pouring fuel on the fire, not putting it out. Protective genes are turned off and inflammatory genes are turned up. I also think that
parabiosis experiments provide a strong clue. Three researcher groups (at Stanford Harvard, Berkeley) have shown that injecting blood plasma from a young mouse into an old mouse makes the old mouse healthier, and relieves some problems associated with age. The blood plasma contains no cells—only signal molecules that are the product of gene expression. This is powerful evidence that youthful gene expression is supporting a strong and youthful body, and (conversely) that the kind of gene expression that characterizes old age is not doing the body any good.
But the ultimate experiment will be to re-program gene expression in an old mouse and see if there is a rejuvenating effect.
My proposal
As of now, the GILGA-Mesh project is dominated by numbers geeks (like me) who practice the “Google approach” to bioinformatics. Huge databases of gene expression are screened for epigenetic candidates that seem to be well-correlated with good outcomes. I think what we need is an infusion of biolochemists who understand something about the body’s signaling networks, and can orient us toward “upstream” and “downstream” molecules. Here’s my proposed program:
- Repeat Horvath’s (human) analysis for mice. In other words, identify several hundred places where methylation is different in young and old mice.
- Determine which genes are associated with these regions. (Map needed for this should already be available.)
- Look at the set of genes and identify transcription factors. These are likely to be “upstream”, in that they control other genes.
- Start with old mice. Use CRISPR to change the methylation status in a handful of promoter regions that control transcription factors, making them match the methylation status of young mice.
- Measure metabolic functions to see if the old mice are more healthy or less after these procedures. Look particularly for changes in inflammation, propensity for cancer, and especially life span.
If this experiment goes as I expect, we will be ready for rejuvenation experiments in humans.
How does the body know how old it is?
Even further upstream, is there a central master clock that dictates the body’s epigenetic expression, and thereby determines our biological age? Logically, it seems that the body would need an accurate clock to time the events of growth and development. Evolution likes to re-use the parts she has created, and it would not surprise me if the developmental clock morphs into an aging clock.
I have reasoned that there are two possibilities. It may be that there is a timekeeper, probably in the neuro-endocrine regions of the brain, that controls the processes of development and aging. This possibility is supported by works of Kasper Daniel Hansen and Claudia Cavadas. If this pans out, it would present the handiest target for true rejuvenation in humans. But it also may be that epigenetic expression itself is a kind of clock that is diffused through the body. Today’s gene expression includes transcription factors that control tomorrow’s gene expression, and so epigenetic state may be a feedback loop, or self-contained clock. This may also be a target for rejuvenation, but a little accessible, harder to address or to tinker with.
Random notes—other things I learned last week
I was tickled to find how many members of the GILGA-mesh team already support the
programmed aging perspective that I have advocated. I was particularly gratified to receive encouragement from Caleb Finch, a grand old man of the field who wrote the
encyclopedia of aging in 1990, and continues a very active research program today.
From Finch, I learned that infections in childhood and even in the womb can have a serious effect on diseases of old age, decades after the fact. He hypothesizes a lifelong burden of inflammation. Evidence includes an elevated incidence of heart disease for the cohort born just after the influenza epidemic of 1918.
I was chagrined to learn that air pollution, especially particulate matter, is associated with increased risk of dementia. This poses a personal dilemma for me, as I plan to spend the summer at the lab of Meng-qiu Dong in Beijing.
I learned that hospital errors are the third leading cause of death in the US, accounting for about 10% of all deaths, about the same number as smoking. Maybe you already read that in the New York Times.
Discussion
74 reader comments
Imported threads are marked Archive. New comments are welcome and moderated for spam.
It would be interesting to find evolutionarily conserved regions of epigenetic clock CpG methylation - that are changing in the same way in humans, mice, rats, dogs, cats, cows, etc. during aging.
Furthermore, in addition to the plan.of Josh Mitteldorf
It would be nice to try to start the epigenetic reprogramming of human blood cells by separating them from the plasma, and then transfer these blood cells to the young donor plasma (in parallel with the forced by dCas9-activator transcription activation of genes that were working in the young blood and dCas9-TET1 selective demethylation).
In support of Josh Mitteldorf proposed program:
Even a non-specific action on DNA methylation (experiments with 5-azacytidine - inhibitor of DNA methyltransferase enzyme, Dnmt1), http://www.pnas.org/content/113/16/E2306.abstract allows to reprogram the cells in vitro into safe tissue-regenerative multipotent stem cells. Another DNA methyltransferase inhibitor, RG108 significantly induces the expression of TERT by blocking methylation at the TERT promoter region. Under RG108 treatment in human bone marrow mesenchymal stromal cells, the anti-senescence genes TERT, bFGF,VEGF, and ANG were increased, whereas the senescence-related genes ATM, p21, and p53 were decreased. Number of senescence-associated β-galactosidase-positive cells was significantly decreased. (http://onlinelibrary.wiley.com/doi/10.1002/bab.1393/full?elq_mid=6940&elq_cid=1845997)
I was at a party this last weekend and talked to a man with Parkinson's Disease. Since there is only a week link to genetics could this be a result of corruption of the epigenome?
I talked to a woman who said she was allergic to whey protein. She said her doctor told her that the reason she was allergic was because she is Swiss and has consumed a huge amount of dairy her whole life. The doctor told her that if a person was to consume several carrots a day that by the time they were well into adulthood they too would generate an allergy to carrots. I told her that this did not fit the allergy model. Are the whey and gluten intolerant suffering epigenetic or microbiome problems?
Ontogeny recapitulates philology! I asked a doctor friend two decades ago how the code that made us up was changed to produce the various organs in our bodies. He said the DNA was edited and implied that different DNA was in our skin and liver. Hail epigenome! You have mentioned that you think in numbers and code. I am thinking we are going to have added difficulty because the epigenome is not a single code overlaying all of our DNA but different code with different aging sequences within the different types of cells in our body. Am I right?
Hi Josh I truly admire how well you try to give a 3D perspective of a topic without any bias. No wonder you have so many readers and fans. I agree with this post that evidence is clearly leaning towards programmed aging across all living. One of the latest developments which can be cited towards this is argument is the discovery made by Hayashi and his team at Tsukuba University. No difference in DNA damage between a foetus, 12 year old or a 90 Year old. A lot of anti aging research by very important scientists is based on trying to attenuate the symptoms of aging via telomeres/telomeradr or NAD+ or glycine replenishment. This may give small benefits but won't lead to a cure of aging. We are constantly run by a software right from the time we are in the womb forming our body parts to a fast growing baby to an adolescent hitting puberty to aging and death. It is difficult to believe that a software program runs making big and subtle changes to us only till we reach adulthood and then abruptly stops and then wear and tear becomes the cause of changes. It is so obvious that our entire life cycle is a coded program. Survival of species may be what has patterned this program. Whether it is cancer cells, humans or trees there are various mechanisms adopted to optimize our chances of survival. The day we as a species reach a point where we do not need a bio-chemical program to survive we will discover the cure to aging. Of all the species we are the closest. Fascinating times we live in.
I am in a position to raise funding from investors for experiments mentioned by Harold Katcher (HPE on humans via plasmaperesis) and what Josh you mentioned in this post because of my background in investment banking and private equity. I have access to HNIs old timers and family offices who would invest to be first in que if the experiments succeed. Will hope that something good emerges out of such research and experiments in our lifetime as it is a shame that a human that accumulates and evolves knowledge over years to then turn into rotting flesh in a short span.
If you are willing to help raise funds, here are three projects I would offer as underfunded and very promising:
1) Telomerase activation strategies. Screening chemicals in vitro, then testing them in vivo.
2) Plasma transfusions. I would like to see an 80-year-old receive transfusions of blood plasma from 20-year-olds, perhaps once a week for several months. If there are dramatic results, this would attract new research and investment in the field.
3) Testing known anti-aging treatments in combination in rodents. We know only about action of treatments one-at-a-time. If these 10% and 20% benefits can add up, that would be great. But I think it likely that most combinations won't work that way. Let's do a broad search for combinations that synergize. There is a crowd-funded group at MMTP which I am already in touch with, and I have a proposal in need of funding. Because of economies of scale, this would need to be funded with several hundred thousand dollars to produce results, but those results would be enormously valuable. https://scienceblog.com/joshmitteldorf/2015/12/22/we-know-nothing-about-longevity-drug-interactions/
Lolz Josh, what took Harold so long to bring this to your attention? I think you should be glad I don't "turn off the computer and spend time with" monkeys after all, heh? ;-)
Josh,
ad. 2)
A company called Amborisa is already starting clinical trilas with parabiosis. Amborisa is apparently being financially backed by Peter Thiel.
http://www.dailymail.co.uk/sciencetech/article-3718758/Peter-Thiel-believes-blood-transfusions-young-key-living-forever.html
Yes would love to contribute in a research project of mutual interest.
1. I am not a big fan of Telomeres and Telomerase path to Longevity - the idea is to upstream as much as possible and Telomeres are as downstream as one can get. although I don't know what you think of BioViva's claim of lengthening the Telomeres of their CEO. Personally I do not see a cure for aging coming from interventions aimed at the symptoms of aging.
2. Parabiosis and may be HPE have an intriguing prospect. Any coding needs to transmit it's code to multiple targets for execution. Parabiosis offers prospects of swapping this message in transit. We can try and mobilize funding for HPE and tinker around the methodologies to see if it works but we will need to provide verification to our investors for which Steve Horvath's DNA methylation lab would be required.
3. I agree testing known anti aging interventions in various permutations and combinations may lead to valuable results.
I am already in the process of funding an anti-aging clinic and lab and one of the key focus areas is to discover and bank combinations that ensure bioavailability. My guess is that 95% of supplements fail because of poor absorption rates. We are only looking at natural compounds or occurring in our body (which need augmenting due to decline with aging). So rapamycin and metformin will not be part of our offered therapies. An average person who has begun to age is not aware of all the safe interventions which have reasonable body of evidence and may allow for mitigation of some of the onslaught of aging - so at this clinic we hope to offer the most comprehensive portfolio of anti aging interventions which would be further tested at our labs for bioavailability, efficacies and safety.
Would be happy to discuss over email what we can target jointly for funding while keeping in mind that investors will expect program that may lead to a commercial outcome and not just a knowledge building outcome.
@ Akshay - you can also look at CyGenia:
http://www.cygenia.com/?q=en/epigenetic-services/biological-age
they offer services to measure biological age.
Thank you Adrian that was useful. I was not aware of non invasiveoption.
To Charles Kendrick
Yes, I did not doubt your citation on the effect of telomere elongation in mice. I just dismissed it when I had read it earlier and then forgot about it.
The reason of my dismissal was that like many interventions, I feel it is just palliative, somehow reducing the burden of old age, but does not fundamentally extend lifespan. I think the same about mTOR/IGF1/GH related findings and senolytics, too. As I wrote before I would like to see a mouse that ages like a cat before I believe anything significant had been found.
Also in my view telomere elongation is really downstream. Adult stem cells are supposed to elongate their telomeres to live and divide for decades.
http://www.uam.es/personal_pdi/ciencias/depaz/adi/internet/ecr_ejercicio_4_Meshorer_Blasco.pdf
Telomere erosion in differentiated cells shouldnt matter as there is ample supply of new cells from stem cells.
Non dividing cells do age, too, and telomeres should not shorten in non dividing cells. Also telomere length shows a very noisy correlation with aging.
https://scienceblog.com/joshmitteldorf/2015/04/29/large-new-survey-tracks-telomere-length-and-mortality/
Yes, you are correct that DNMT KO is lethal very early on.
http://file.scirp.org/pdf/SCD_2013042315273513.pdf
I could not really find anything about someone upregulating DNMTs. The general thought is that these are oncogenes because they are upregulated in many cancers. There are cancer drugs targeting DNMTs
http://www.ncbi.nlm.nih.gov/pubmed/23898051
However I would not link increased DNA methylation with cancer, I think its probably about selective methylation of onco suppressors.
I would be really glad if I could read about research with overexpressing DNMTs.
General DNA hypomethylation also helps cancer (in my view this is the primary reason for increased cancer incidence with age)
http://www.ebioe.com/uploadfile/201106/20110607103903730.pdf
And when I wrote about transcription profile I was referring to the link cited by Josh about Steve Horvath's research.
http://www.nature.com/news/biomarkers-and-ageing-the-clock-watcher-1.15014
He was trying to find differences in the transcritption profile of old vs young somatic cells and he found none. This is very strange since we know he discovered a very specific aging pattern in DNA methylation.
In this wonderful 2002 paper
http://mcb.asm.org/content/22/7/2124.full
the authors overexpresed DNMT1 by 250% (measured by methyltrasferase assay) in ES cells. The 5mC content hardly raised but there were adverse and embryonic lethal side effects.
My understanding is that DNMT1 level in ES cells is saturated so overexpression there does not help anything only makes things worse. Would love to see an analysis of methyltransferase activity in old differentiated and adult stem cells vs young and also DNMT overexpression there.
I agree with you GaborB most of the research today is towards palliative solutions and not upstream enough. Thank you for the link to Benayoun, Polina, Brunet paper
Hi Josh,
what if the epigenetic clock is driven by wear and tear? I mean wear and tear of the DNA methylation state? This would be quite logical. DNA methylation state is reset at embryonic development only. Then it is a one way road for most of the cells. They go from totipotency to senescence, from undifferentiated to differentiated state.
Aging is characterized by a generic, random demethylation of the DNA and methylation at specific sites (bivalent chromatin - genes switched on and off by PRC complex)
Do we have a repair mechanism if a CpG site becomes demethylated on both strands by accident?
I know of only single strand repair (DNMT1 - needed for maintaining methylation state at mitosis) and de novo methylation (DNMT3a and b).
We know organismal aging is correlated with DNA methylation. We also know maximum lifespan is correlated with free radical production by mitochondria when comparing different species.
What if the two are related? What if the wear and tear hypothesis is correct but not against the DNA or cellular organelles, but the DNA methylation state - which is reset only in embroynic age.
And what if this is more than sufficient for maintaining a diversity of lifespans across species spanning from weeks to hundred years? I mean its enough to satisfy population dynamics requirements set by the niche the species living in?
Interesting read on methylation maintainance
http://www.ncbi.nlm.nih.gov/pmc/articles/PMC1203935/pdf/ge1242429.pdf
It's the 2nd time I see you crediting Francis Crick in this blog, Josh. (and I think I saw Harold do it on the previous comment section as well.. of all people.. 'cause it's not enough to live forever, we also gotta have all the glory. : ) Just kidding Harold, still love ya.. even if you don't gimme any credit ^__^)
I cued up an interesting piece of information for you here: https://youtu.be/j7EBObU5Tjk?t=33m48s
Symbolism is extremely important btw ; ) and shall only become ever more so.
The link about Steve Horvath was especially interesting. (Can we read about that brain storming session anywhere btw?)
What I find most interesting is that the gene expression profiles yielded no results. I simply cannot believe it. If there is difference in the phenotype between old and young cell, and of course we know there is - there must be difference in the expression profile as well - or the whole direction of research you and others follow is dead end. I can hardly think of an aging program that does not show up in transcribed or translated products.
Maybe they looked at some sparse RNA chip data only and not deep whole transcriptome sequencing?
C. Elegans nematode worms are studied as model organisms because of their simplicity. It seems an organism doesn't have to be very complicated to have a clock.
http://cmgm.stanford.edu/~kimlab/index_wormaging.html
Nice post. As far as I know, there is no direct evidence suggesting a possible impact of telomere lenght on methylation levels in cells, so I would like to know more about this subject. Is there any hint in current literature? Thanks. Hope to hear from you.
Telomere length affects gene expression, but not through methylation. It's called the telomere position effect, TPE. Google it.
- Josh
That's was exactly what I was thinking about. Thanks, Josh.
Hi Josh.
I'm curious as to what evolutionary mechanism you see driving the epigenetics of aging? Also, through-out most of human history our ancestors had a much shorter life span than modern man. What opportunity would there be for a mechanism that would have had to evolve over millions of years to occur, if human life span has been brutally short?